Pre-synaptic terminals of glutamatergic neurons retrieve a portion of the glutamate released in response to incoming action potentials
The cell membrane of these terminals contain excitatory amino-acid transporters ( EAAT ) , along with transporters such as Na+/K+-pumps , K+ channels , and likely Na+/H+ exchangers
The coupling stoichiometry of EAAT is cotransport of one glutamate with 3 Na+ and one H+ ,
all in exchange for one K+
You assume that the basal condition of the pre-synaptic terminal under study has the following properties :
You predict that high synaptic activity will enhance the driving force for glutamate uptake
Draw a diagram of the pre-synaptic terminal that includes EAAT and the other transporters needed to achieve a steady-state
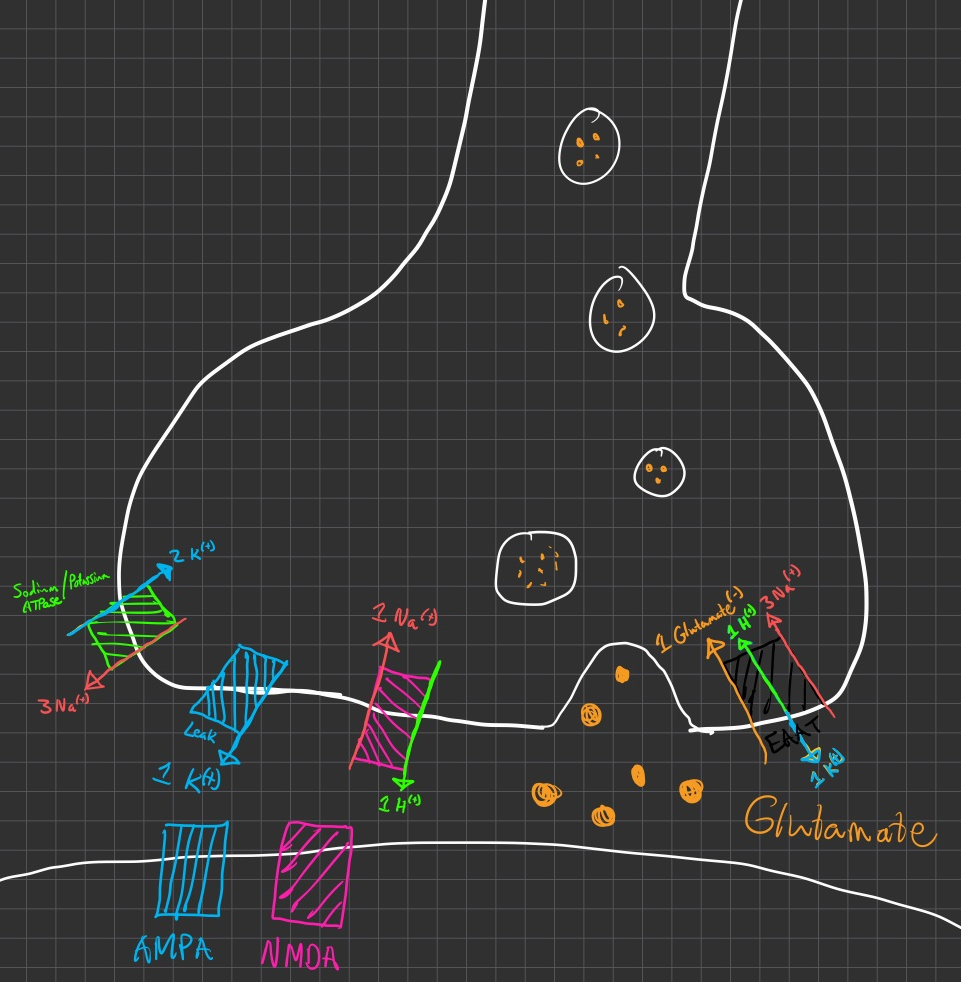
EAAT Net Charge = +2 charges moving inside
In the absence of incoming action potentials, glutamate at the pre-synaptic terminal is :
and
For the resting condition , calculate the driving force for EAAT ( and flow direction )
| Ion | Contribution ( | |||
|---|---|---|---|---|
| Na | 3 | +1 | ||
| K | 1 | +1 | ||
| H | 1 | +1 | ||
| Glutamate | 1 | -1 | ||
| 1 | +2 |
Calculate the driving force for EAAT at the peak of an incoming action potential
let peak action potential
| Ion | Contribution ( | |||
|---|---|---|---|---|
| Na | 3 | +1 | ||
| K | 1 | +1 | ||
| H | 1 | +1 | ||
| Glutamate | 1 | -1 |
High frequency action potential arrival in the terminal excites glutamate release such that :
and
Calculate the driving force for EAAT during these inter-spike periods and at the peaks of these action potentials
Inter-Spike Periods
| Ion | Contribution ( | |||
|---|---|---|---|---|
| Na | 3 | +1 | ||
| K | 1 | +1 | ||
| H | 1 | +1 | ||
| Glutamate | 1 | -1 |
At Action Potential Peak
| Ion | Contribution ( | |||
|---|---|---|---|---|
| Na | 3 | +1 | ||
| K | 1 | +1 | ||
| H | 1 | +1 | ||
| Glutamate | 1 | -1 |
Hypoxic conditions stress the pre-synaptic terminal altering the ion gradients :
|| || ||
Determine the reversal potential for EAAT during these hypoxic conditions.
| Ion | Contribution ( | |||
|---|---|---|---|---|
| Na | 3 | +1 | ||
| K | 1 | +1 | ||
| H | 1 | +1 | ||
| Glutamate | 1 | -1 |
Astrocytes adjacent to pre-synaptic terminals of glutamatergic neurons also retrieve a portion of the glutamate released in response to incoming action potentials.
These astrocytes convert glutamate to glutamine and then extrude glutamine for retrieval by pre-synaptic terminals ( glutamine-shuttle ) , such that post-synaptic glutamate receptors remain unaware
Cell membranes of these astrocytes contain Na+-dependent neutral amino-acid transporters ( SNAT3 ) , along with transporters such as Na+/K+ pumps , K+ channels , and likely others
The coupling stoichiometry of SNAT3 is cotransport of one glutamine with one Na+ in exchange for one H+
Cell membranes of these pre-synaptic terminals contain SNAT1
The coupling stoichiometry of SNAT1 is cotransport of one glutamine with one Na+
You assume that for the synaptic locale under study , the basal condition has the following properties :
You predict that extracellular glutamine concentrations will remain in a narrow range that supports continual glutamine uptake by the pre-synaptic terminal
Draw a diagram of the synaptic locale that includes SNAT and the other transporters and enzymes needed to achieve a glutamate re-supply for the pre-synaptic terminal
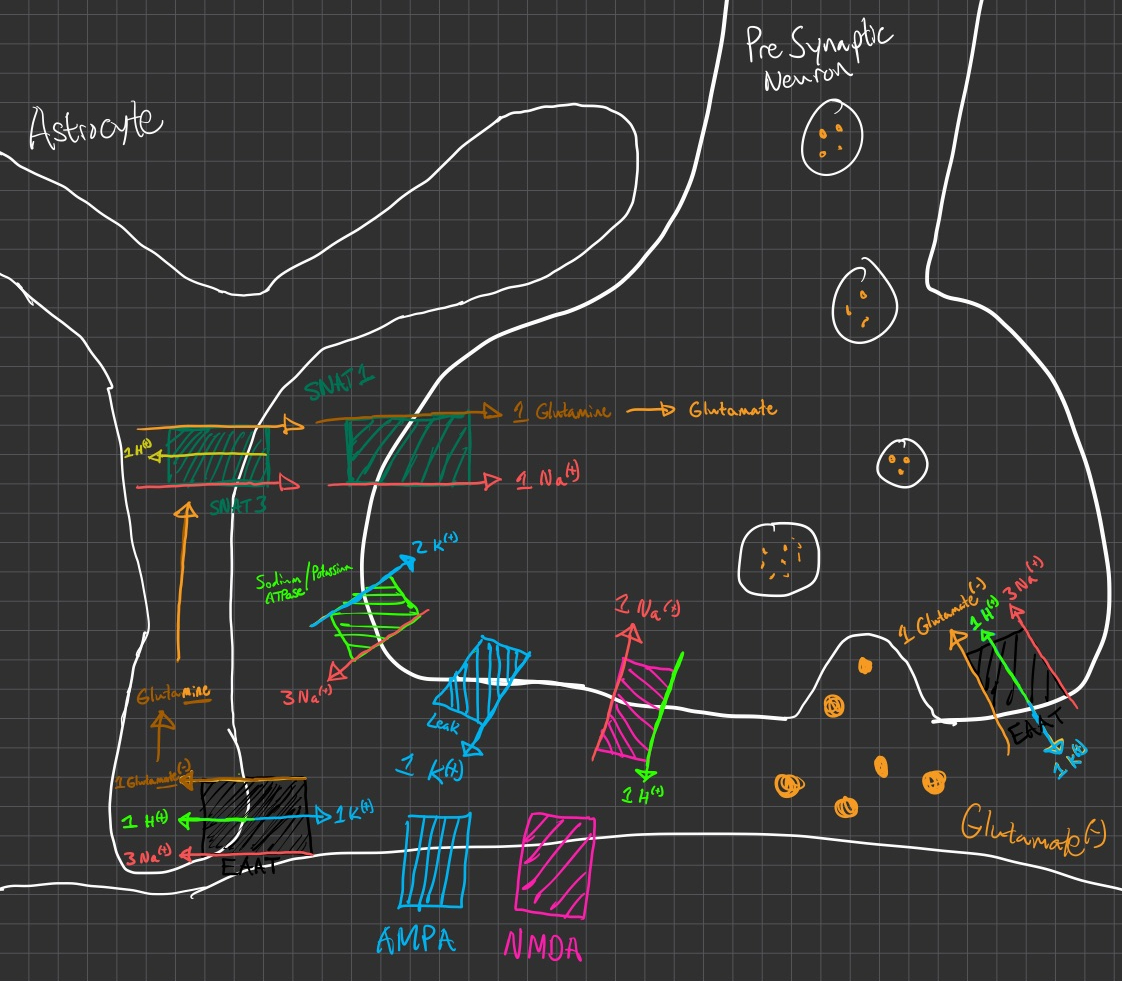
Calculate the driving force for SNAT1 and for SNAT3 during the inter-spike periods
SNAT1
| Ion | Driving Force | Contribution ( | |||
|---|---|---|---|---|---|
| Na | 1 | +1 | |||
| Glutamine | ? | 1 | 0 |
SNAT3
| Ion | Driving Force | Contribution ( | |||
|---|---|---|---|---|---|
| Na | 1 | +1 | |||
| H | 1 | +1 | |||
| Glutamine | ? | 1 | 0 |
Calculate the driving force for SNAT1 and for SNAT3 at the peak of an incoming action potential
let action potential peak =
SNAT1
| Ion | Driving Force | Contribution ( | |||
|---|---|---|---|---|---|
| Na | 1 | +1 | |||
| Glutamine | ? | 1 | 0 |
SNAT3
| Ion | Driving Force | Contribution ( | |||
|---|---|---|---|---|---|
| Na | 1 | +1 | |||
| H | 1 | +1 | |||
| Glutamine | ? | 1 | 0 |
Determine the
SNAT1
| Ion | Driving Force | Contribution ( | |||
|---|---|---|---|---|---|
| Na | 1 | +1 | |||
| Glutamine | ? | 1 | 0 |
SNAT3
| Ion | Driving Force | Contribution ( | |||
|---|---|---|---|---|---|
| Na | 1 | +1 | |||
| H | 1 | +1 | |||
| Glutamine | ? | 1 | 0 |
Hypoxic conditions stress the synaptic locale altering the ion gradients :
|| || || ||
Determine the range of